FIG. 86Senses
How do bats see with sound? Echolocation explained
An echo from a moth 1 m away comes back to a bat in under 6 thousandths of a second, and that delay is how the bat knows the distance.
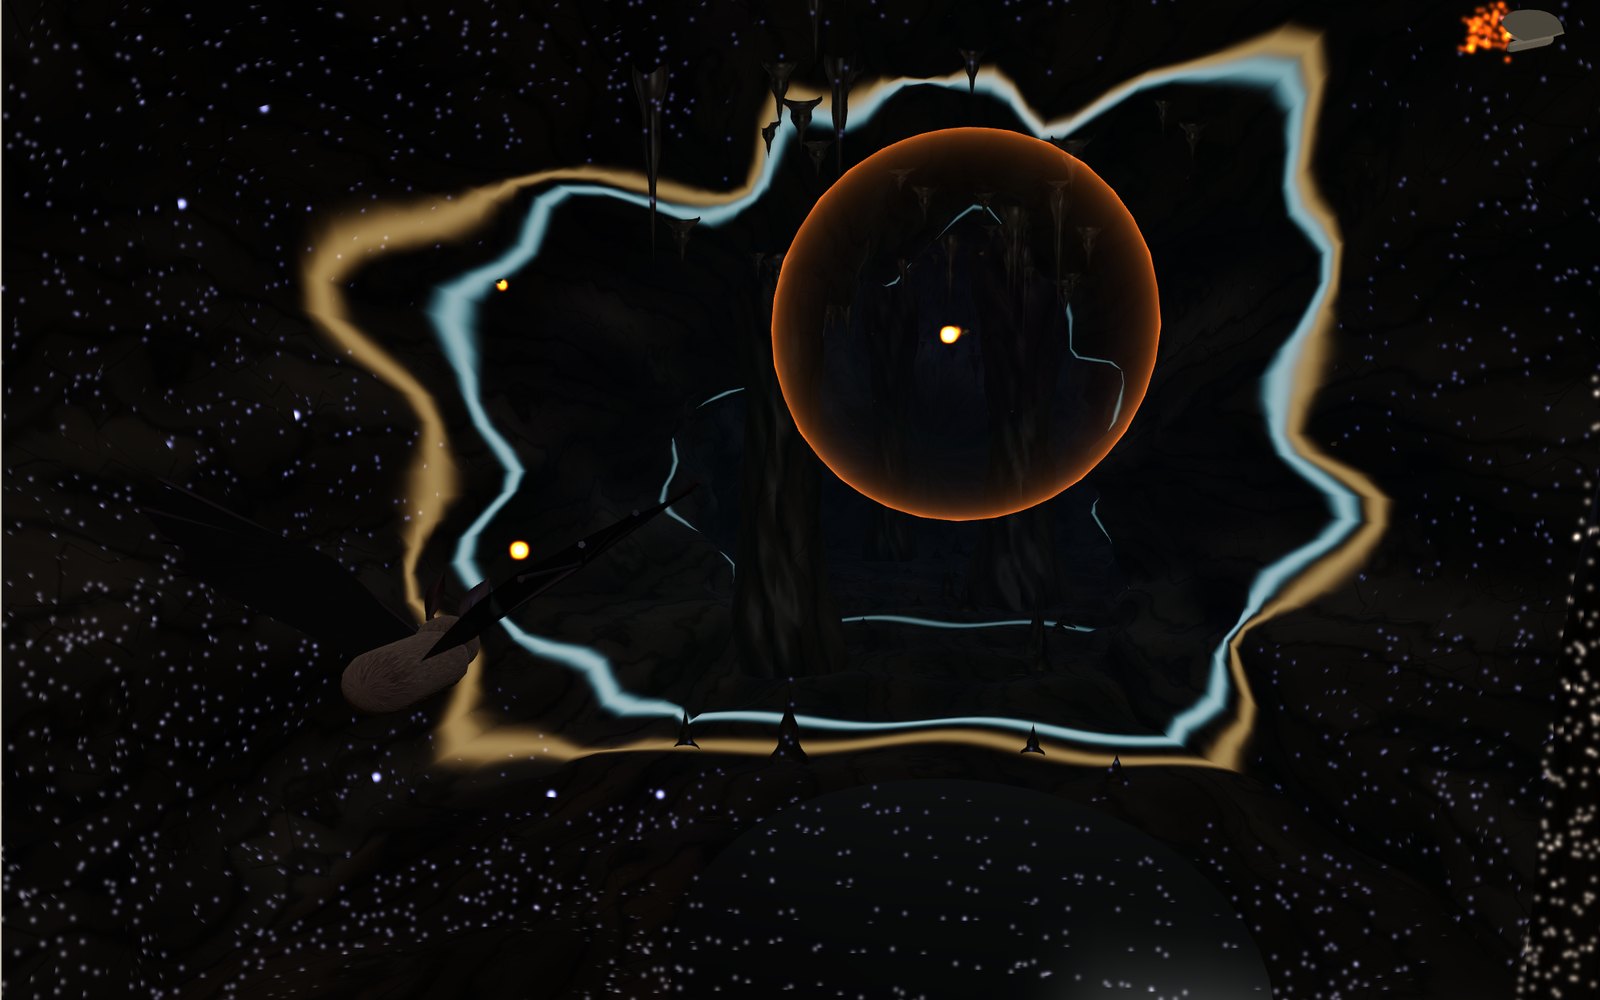
This device cannot show the 3D model. You can read the guide steps below as text.
1 / 10 A cave with no lightThere is no light in this cave. The bat has sent one call; the bright shell is the sound spreading out at 343 m/s. Tap Click to call again, or follow these steps.
Drag to turn. Scroll or pinch to zoom.
A clap in a dark hallway
Stand in a long, empty hallway with your eyes closed and clap once. You hear the clap, then a faint copy of it a moment later, and you get a rough sense of how far away the far wall is. A bat does the same thing hundreds of times a minute, with sounds too high for us to hear, and it does it well enough to catch a moth in flight in total darkness.
This is called echolocation: send out a sound, listen for what comes back, and work out from the echo where things are and what they are like. This exhibit puts you in a limestone cave with no light at all. A big brown bat calls, and you can watch each call spread through the cave, bounce off walls, columns, drips and insects, and come back. When an echo gets home it becomes a glowing point. After a few seconds those points add up to a picture of the cave, and that picture is the only one the bat has.
How to use the stage
Press Click to make the bat call once. The bright shell is the front of the sound, drawn brighter where the bat is aiming. When the shell reaches something solid, an amber shell may start back from it, and when the echo arrives at the bat a point appears in the echo map. Warm points are close, blue points are far, and orange points are moths. Points fade after the time set by the Echo memory slider.
The buttons under the stage set the slow motion. Sound in air covers 343 metres in a second, so a whole call and all its echoes would be over before you could see anything. At 100 times slower the call crawls along at about 3.4 metres a second. Hunt the moth sends the bat after the nearest moth at real flying speed (shown 10 times slower), and the call rate rises on its own as it closes in.
In the Controls pane you can change the bat species, set the hunting phase by hand, stop the automatic calling, turn on the sound, show the Doppler shift of the moth's echo, let the moth jam the sonar, switch on a lamp, and show the sonar beam. Under the controls an echo calculator does the arithmetic of this page for any distance, temperature and frequency. Under the stage is a list of 34 animals and machines that find things by echo.
Distance from a delay
The rule at the centre of echolocation is short. Sound travels at a known speed. If an echo arrives a time t after the call went out, the sound has gone to the target and back, so the target is at
distance = speed of sound × t ÷ 2
In dry air the speed of sound depends on temperature. It is the square root of 1.4 × 287.05 × T, where T is the temperature in kelvin. At 20 °C that gives 343.2 m/s. At 0 °C it is 331.3 m/s, and on a 30 °C summer night it is 349.0 m/s. A bat in a cold cave and a bat over a warm meadow live with slightly different rulers, about 5 percent apart.
With 343.2 m/s, the echo delays come out like this:
| Distance | Echo delay |
|---|---|
| 10 cm | 0.58 ms |
| 1 m | 5.83 ms |
| 3 m | 17.48 ms |
| 5 m | 29.14 ms |
| 10 m | 58.27 ms |
| 20 m | 116.54 ms |
So the column 10 metres ahead of the bat answers after about 58 thousandths of a second, and the moth 3 metres away after about 17. A difference of one microsecond in delay is a difference of only 0.17 mm in distance. Bats cannot use timing that fine, but experiments by James Simmons in the 1970s showed that trained big brown bats could tell which of two targets was nearer from the echo delay alone.
On the stage the time is real: every point is drawn at the moment its echo would arrive, scaled by the slow motion. Watch a call reach the far end of the tunnel and you will see the far points light up last.
Why the calls are so high
Most bat calls are ultrasonic, above the roughly 20 kHz limit of human hearing. The big brown bat on the stage sweeps down from about 50 kHz to 25 kHz in a few milliseconds. The common pipistrelle is loudest near 45 kHz and the greater horseshoe bat holds a tone near 82 kHz.
The reason is the size of the wave. The wavelength is the speed of sound divided by the frequency. At 10 kHz it is 34 mm, at 35 kHz about 10 mm, at 82 kHz about 4 mm. A target much smaller than the wavelength hardly disturbs the wave and sends back very little; the echo from a small sphere falls roughly with the fourth power of the ratio between size and wavelength. A mosquito is a few millimetres long. To get a strong echo from it a bat needs a wavelength of a few millimetres too.
High frequencies have a cost. Air absorbs sound, and it absorbs high frequencies much more. Using the standard formula for absorption in air (ISO 9613-1) at 20 °C and 50 percent humidity, the loss is about 0.16 dB per metre at 10 kHz, 0.52 dB at 20 kHz, 1.13 dB at 35 kHz, 2.67 dB at 82 kHz and 3.28 dB at 100 kHz. The echo pays that price twice, going out and coming back. At 100 kHz a target 5 metres away loses 33 dB to the air alone.
Turn the Bat slider from the big brown bat to the greater horseshoe bat and watch the echo map: the high tone draws a sharper but shorter map. Turn it to the spotted bat, which calls at 9 to 12 kHz, and the map reaches deep into the tunnel but every point is fuzzier.
How loud, and how far
Bats are loud. Field recordings in Panama by Annemarie Surlykke and Elisabeth Kalko found source levels of 122 to 134 dB SPL, measured 10 cm in front of the bat, for bats hunting in the open. Two species that hunt over water averaged about 137 dB and reached above 140 dB. We do not hear any of it only because it is too high.
They need to be. A sound spreading in all directions loses 6 dB every time the distance doubles. The echo spreads again on the way back, so the round trip loses 12 dB per doubling of distance. A moth reflects only a tiny part of what hits it. The model on the stage uses the sonar equation:
echo level = source level − 40 log₁₀(r ÷ 0.1 m) − 2 × absorption × r + target strength
With a call of 120 dB at 10 cm, a moth target strength of −30 dB and a hearing threshold of 20 dB, the bat in the model hears a moth to about 3.5 m at 35 kHz, 3.1 m at 50 kHz and 2.6 m at 82 kHz. A rock wall returns far more, so it can be heard to about 8 m at 35 kHz. These are model numbers, but they match the field picture: prey is found at a few metres, walls and trees at several times that. Surlykke and Kalko also noticed that the loudest bats used the highest frequencies, which seems to bring their detection distances back into line with the others.
The Moth heard to line on the stage readout shows this model distance for the bat you have chosen. The moth only turns orange in the echo map when it is inside that range.
Search, approach and terminal buzz
Around 1960 Donald Griffin and his colleagues recorded bats hunting insects and found the calls change in a regular way. While searching, a big brown bat calls about 10 times a second, each call several milliseconds long. Many bats call once per wingbeat in this phase, so flapping, breathing and calling share a rhythm. When it detects an insect it enters the approach phase: the calls get shorter and come faster. In the last few hundred milliseconds comes the terminal buzz, when the rate rises past 160 calls a second and the calls shrink to well under a millisecond.
One part of the reason is simple timing. A bat usually waits for the echo it cares about before it calls again, so that echo and call do not overlap. From 5 metres the echo takes 29 ms, which allows at most about 34 calls a second. From 1 metre it takes 5.8 ms, which allows 172. From 50 cm it allows 343. The closer the prey, the faster the bat is allowed to call, and the more often it learns where the moth has moved.
That is not the whole story. In 2011 Coen Elemans and colleagues found that bats have superfast muscles in the larynx, among the fastest muscles known in mammals, and that the top call rate is set by how fast those muscles can work, not only by echo overlap. Set the Hunting phase slider to Terminal buzz and the shells pour out of the bat so fast that they nest inside each other.
Which direction: two ears
Distance comes from time. Direction comes from comparing the two ears. An echo from the right reaches the right ear a little before the left one, and it is also a little louder there, because the head shades the far ear. In the model the ears are about 1.6 cm apart, so the largest time difference, for an echo straight from the side, is about 47 microseconds. An echo 10 degrees off centre gives about 8 microseconds. The readout prints this difference for the moth.
Up and down are harder, because both ears are at the same height. Here the shape of the outer ear helps. The small flap in front of the ear opening, the tragus, adds its own echo inside the ear, and the timing of that tiny extra echo depends on whether the sound came from above or below. Bats also move their heads and ears between calls, and with each call they hear the scene from a slightly different angle. The bat on the stage turns its head a little between calls, which is how its map fills in.
Doppler: is the moth coming closer?
When the bat flies toward a wall, each wave crest of its call is sent from a little closer than the one before, so the wall receives a slightly higher frequency. The wall then sends that sound back to a bat that is still approaching, and the frequency rises again. For a bat flying at speed v toward a still target, the echo comes back at
f × (c + v) ÷ (c − v)
At 4 m/s an 82 kHz call returns at about 83.9 kHz, almost 2 kHz higher. If the target is moving too, its own speed adds in the same way. Turn on Doppler shift and the readout shows the frequency of the moth's echo and how far it is from the call.
Horseshoe bats make the most of this. Their call is a long, nearly constant tone, and their hearing has a narrow band of very sharp tuning near their echo frequency, sometimes called an acoustic fovea. As a horseshoe bat flies forward it lowers its call by just enough that the Doppler-shifted echo lands in that band. At 4 m/s it calls at about 80.1 kHz so that the echo returns near 82 kHz. Against that steady tone, the beating wings of an insect make the echo flicker in pitch and loudness, and the bat can pick out a fluttering moth among still leaves. Choose the greater horseshoe bat on the Bat slider to see the numbers.
What echoes say about surfaces
Rough rock scatters sound in all directions. Wherever the beam lands, some of it comes straight back, which is why the cave walls fill with points. A smooth surface acts like a mirror instead. The call bounces off at the same angle it arrived and travels away, and only the part of the water directly below the bat sends an echo back.
That is why the pool on the stage stays dark in the echo map. Stefan Greif and Björn Siemers showed in 2010 that bats treat any large, acoustically smooth surface as water. Wild bats of 15 species tried to drink from smooth plates of metal, wood and plastic, even when the plates were in plain view. Young bats that had never seen water did the same, which suggests the rule is inborn. On the stage, the pool shows up as a hole in the map with a single bright spot beneath the bat.
Moths fight back
Moths have been hunted by bats for tens of millions of years, and many have answers. A large share of moths have ears that hear bat calls. When a call gets loud they dive, loop or drop to the ground. Some bats in turn call at frequencies those ears hear poorly, or call very quietly. The brown long-eared bat is known in Britain as the whispering bat.
Some tiger moths answer back. In 2009 Aaron Corcoran, Jesse Barber and William Conner filmed big brown bats attacking the tiger moth Bertholdia trigona in the dark. When the bat entered its terminal buzz, the moth produced dense bursts of ultrasonic clicks, and the bats missed. The clicks seem to confuse the bat about how far away the moth is. Turn on Moth jams sonar and start a hunt: the moth's echo smears into red points at the wrong distances, and in this model the bat usually overshoots.
Luna moths use another trick. Their long hindwing tails spin as they fly and return echoes of their own. In experiments by Barber and colleagues, bats aimed at the tails in more than half of their attacks, and moths with tails survived about 47 percent more often than moths without. Bats also jam each other: Mexican free-tailed bats chasing the same insect make a special call that makes the rival miss.
Other animals that echolocate
Bats are the best known, but not the only ones. Toothed whales, including dolphins and porpoises, echolocate under water, where sound travels about 4.4 times faster than in air. Their clicks are short and very loud. On-axis clicks of sperm whales, recorded by Bertel Møhl and colleagues, reached 236 dB re 1 µPa, the loudest sounds known from any animal. Peter Madsen and Annemarie Surlykke have shown how closely the sonar of bats and toothed whales converged, even though the two groups evolved it separately.
Two kinds of birds echolocate too. The oilbird of South America eats fruit at night and nests deep in caves, and the cave swiftlets of the Indo-Pacific nest in dark caves as well. Both use clicks low enough for people to hear, which carry well but show less detail. Shrews twitter more when they explore cluttered places, and recordings suggest their calls give useful echoes at short range. Even some fruit bats long thought not to echolocate find their way in the dark with clicks made by their wings.
People who echolocate
Some blind people echolocate with mouth clicks. In 2011 Lore Thaler, Stephen Arnott and Melvyn Goodale scanned the brains of two blind experts while they listened to recordings of their own clicks and echoes. The echoes activated the part of the brain that normally handles vision, not extra auditory areas. A 2021 training study at Durham University taught blind and sighted adults aged 21 to 79 to click-echolocate in 20 sessions over ten weeks. Both groups improved a great deal, and neither age nor blindness limited how fast they learned.
Human clicks are a few kilohertz, so their wavelengths are around 10 cm. That is enough to sense a wall, a doorway or a parked car, but not a moth.
Machines that do the same
Ships use sonar, which works on the same rule as the bat with the speed of sound in water, about 1,500 m/s. An echo from a seabed 10 m down returns after about 13 ms. Medical ultrasound sends sound in the megahertz range into the body, where its millimetre-scale wavelengths can show the outline of organs and the heart. The parking sensors in a car bumper use ultrasound to time echoes and find obstacles from about 15 cm to 5 m.
A short history
In the 1790s Lazzaro Spallanzani found that blinded bats still flew without hitting things, and Louis Jurine showed that bats with their ears blocked could not. Nobody could explain how, since the bats seemed silent. The answer had to wait for a microphone that could hear ultrasound. In 1938 Donald Griffin, then a student at Harvard, brought bats to the physicist George Pierce, who had built an ultrasonic detector. With Robert Galambos, Griffin then showed that bats emit ultrasonic pulses and use their echoes to avoid obstacles, and in 1944 he named the ability echolocation.
What the model simplifies
The bat on the stage stays in place between hunts, so you can look around it. A real bat in search flight never stops. The cave is made of a smooth mathematical shape, and the echoes are found by tracing a few hundred rays through the same shape. Real sound is a wave, not a bundle of rays: it bends around edges and the echoes overlap and interfere. The echo strength comes from a simple sonar equation with a fixed target strength for rock, and the hearing threshold is a single number.
The moths are treated as points. A moth's real echo changes with every wingbeat, which is part of how bats recognise insects. The jamming model is only a picture of the result reported for Bertholdia trigona: the moth's echo appears at the wrong distance. The sound you hear is the call slowed down by the same factor as the picture, so a 40 kHz call at 100 times slower comes out at 400 Hz. Bat detectors sold for fieldwork use the same method, called time expansion.
Reading a millisecond echo
Suppose the air is still and its sound speed is rounded to 343 m/s. An echo delay of 1 ms means a total sound path of 343 × 0.001 = 0.343 m. Half of that is the outward path, so the reflector is 0.1715 m away, about 17 cm. Forgetting the return path would put it twice as far away. This example assumes that the echo follows a direct path back from the target. A reflection that bounces from another wall before returning has a longer path and cannot be interpreted as the same straight-line distance.
Frequency does not enter that distance equation. At the same air temperature, a 40 kHz call and an 82 kHz call have essentially the same travel time to the same target. Their wavelengths differ. Using the rounded sound speed, 343 ÷ 40,000 = 0.008575 m, or about 8.6 mm. That number describes the spacing of successive wave crests, not the minimum insect length the bat can detect. A smaller insect can still return an echo; whether the bat hears it depends on its orientation and reflecting surfaces, the distance, and the background noise. An insect's wings also move during an attack. A fixed spherical target is a useful calculation, not an insect identification rule.
In the Echo calculator, set Air temperature to 20 °C, Call frequency to 40 kHz and Distance to target to 1 m. The displayed speed uses the temperature formula rather than the rounded 343 m/s assumed above, so expect about 5.83 ms and 8.6 mm. Doubling distance doubles delay without changing wavelength. Raising frequency changes wavelength and absorption without doubling delay. These are separate effects that a single picture of a bright echo can otherwise hide.
Why the last buzz is not a faster search call
The review by Ratcliffe and colleagues, How the bat got its buzz, discusses more than the number of sounds in an attack. Some bats lower the fundamental frequency in a second part of the buzz. With the same mouth opening, lower frequency broadens the emitted beam. At close range an insect needs to move only a short distance sideways to leave a narrow beam, so a wider acoustic field of view can help the bat keep tracking evasive prey. This is a trade-off against the usual advantage of shorter wavelengths for small targets, not a contradiction of it.
A working example of 200 calls per second gives 1 ÷ 200 = 0.005 s, or 5 ms between call starts. Sound can travel out and back from about 0.86 m in that interval at 343 m/s. That is an ideal timing calculation, not a guaranteed hunting range. Call duration occupies part of the interval, echoes from the surroundings continue to arrive, and the larynx must relax and contract again. The review reports rates up to about 220 calls per second in some species; 200 is not a universal ceiling.
The stage instead uses a nominal Terminal buzz rate of 170 calls per second, with further limits based on target delay. Its displayed rate may therefore be lower when the moth is far away. It also draws a narrower beam during that phase, whereas the study describes beam broadening in the buzz of particular real species. Use the shells to compare calling intervals, not to infer that every bat narrows its sonar beam before capture. The animated cave does not reproduce the full species-specific changes in call design.
Try a controlled comparison on the screen
Start without hunting. Use Clear echo map, then Click, and follow the first returning shells before the older points build up. Switch the lamp on to compare the actual cave shape with the incomplete echo map. A missing point need not mean missing rock: the beam may not have sampled it, or the return may be too weak. This is different from moving a solid object out of the scene.
For a second comparison, keep the species unchanged and use the Echo calculator to vary only Distance to target. Read Echo delay and Fastest rate without overlap together. A greater distance gives a longer delay and a lower ideal repetition rate. The calculator is independent of the moth's actual position; sliding its distance input does not move the moth. This distinction matters when comparing its numbers with the stage readout.
Finally select Greater horseshoe bat, then return to Big brown bat. The former preset represents a long constant-frequency call, while the latter represents a short downward FM sweep. The real horseshoe bat's narrow auditory tuning helps it detect flutter-related changes against foliage; a broadband FM call provides useful timing information about nearby reflectors. These are different emphases, not mutually exclusive senses. Real horseshoe calls also include frequency-modulated portions. The model's constant-tone label deliberately leaves those details out.
Questions
Can people hear bats?
Most bat calls are above 20 kHz, beyond human hearing. Some species call lower: the spotted bat calls at 9 to 12 kHz, and many people can hear it. Bats also make lower social calls. With a bat detector you can hear the rest.
Are bats blind?
No. Bats have working eyes, and fruit bats in particular see well. Echolocation adds a sense that works in complete darkness and is precise at short range.
How far can a bat hear with echoes?
It depends on the size of the target and the frequency. In the model on this page a moth is detectable to about 3.5 m at 35 kHz and a rock wall to about 8 m. Larger objects and lower frequencies reach further.
Why don't bats confuse their own echoes with other bats' calls?
They often shift their call frequency slightly away from their neighbours', and they listen for echoes at the delay they expect. In crowded caves this is still hard, and some bats deliberately jam rivals when chasing the same insect.
Why are the echoes so much quieter than the call?
The call spreads out on the way to the target and the echo spreads out again on the way back, losing 12 dB every time the distance doubles. The air absorbs more on top of that, and a small insect reflects only a tiny part of the sound that reaches it.
Do all bats echolocate?
Almost all insect-eating bats do. Most Old World fruit bats were long thought not to, but the Egyptian fruit bat clicks with its tongue, and in 2014 two more fruit bat species were found to sense objects in the dark with clicks made by their wings.
What is the terminal buzz?
The last part of an attack, when the call rate rises past 160 calls a second and each call lasts less than a millisecond. The bat gets a fresh update on the insect's position every few milliseconds.
Why does the pool look like a hole in the echo map?
Smooth water reflects the call away like a mirror, so almost no echo comes back. Bats use this as a sign of water, and they will try to drink from any smooth plate.
Do the sounds on this page come from real bats?
No. They are synthesised from the call shape of each species and slowed down by the slow-motion factor, which lowers the pitch by the same factor. That is how time-expansion bat detectors make calls audible.
Do dolphins and bats echolocate the same way?
The principle is the same, and the two groups evolved it separately. Dolphins work in water, where sound is about 4.4 times faster, so their echoes come back sooner from the same distance. Their clicks are much shorter than most bat calls.
Terms
- Echolocation: finding objects by making a sound and analysing the echoes.
- Echo delay: the time between a call and its echo. Distance = speed of sound × delay ÷ 2.
- Ultrasound: sound above about 20 kHz, beyond human hearing.
- FM call: a call that sweeps quickly from high to low frequency, good for measuring distance.
- CF call: a call of nearly constant frequency, good for detecting fluttering wings and Doppler shifts.
- Terminal buzz: the very fast calling at the end of an attack.
- Doppler shift: the change in frequency when the source or the reflector moves.
- Target strength: how much of a sound a target reflects, in decibels.
- Tragus: the small flap in front of a bat's ear opening.
Sources
All addresses were checked on 2026-10-17. PubMed pages answer curl with HTTP 203 and the full page.
- Annemarie Surlykke and Elisabeth K. V. Kalko, Echolocating bats cry out loud to detect their prey. PLoS ONE 3 (2008), e2036. Source levels 122 to 134 dB SPL, above 140 dB for Noctilio. https://pmc.ncbi.nlm.nih.gov/articles/PMC2323577/
- Coen P. H. Elemans, Andrew F. Mead, Lasse Jakobsen and John M. Ratcliffe, Superfast muscles set maximum call rate in echolocating bats. Science 333 (2011), 1885 to 1888. https://pubmed.ncbi.nlm.nih.gov/21960635/
- John M. Ratcliffe, Coen P. H. Elemans, Lasse Jakobsen and Annemarie Surlykke, How the bat got its buzz. Biology Letters 9 (2013). https://pmc.ncbi.nlm.nih.gov/articles/PMC3639754/
- Lasse Jakobsen, John M. Ratcliffe and Annemarie Surlykke, Convergent acoustic field of view in echolocating bats. Nature 493 (2013), 93 to 96. https://www.nature.com/articles/nature11664
- James A. Simmons, The resolution of target range by echolocating bats. Journal of the Acoustical Society of America 54 (1973), 157 to 173. https://pubmed.ncbi.nlm.nih.gov/4738624/
- Brian D. Lawrence and James A. Simmons, Measurements of atmospheric attenuation at ultrasonic frequencies and the significance for echolocation by bats. J. Acoust. Soc. Am. 71 (1982), 585 to 590. https://pubmed.ncbi.nlm.nih.gov/7085967/
- Stefan Greif and Björn M. Siemers, Innate recognition of water bodies in echolocating bats. Nature Communications 1 (2010), 107. https://pmc.ncbi.nlm.nih.gov/articles/PMC3060641/
- Aaron J. Corcoran, Jesse R. Barber and William E. Conner, Tiger moth jams bat sonar. Science 325 (2009), 325 to 327. https://pubmed.ncbi.nlm.nih.gov/19608920/
- Aaron J. Corcoran and William E. Conner, Bats jamming bats: food competition through sonar interference. Science 346 (2014), 745 to 747. https://pubmed.ncbi.nlm.nih.gov/25378624/
- Jesse R. Barber and others, Moth tails divert bat attack: evolution of acoustic deflection. PNAS 112 (2015), 2812 to 2816. https://pmc.ncbi.nlm.nih.gov/articles/PMC4352808/
- Hannah M. ter Hofstede and John M. Ratcliffe, Evolutionary escalation: the bat-moth arms race. Journal of Experimental Biology 219 (2016), 1589 to 1602. https://pubmed.ncbi.nlm.nih.gov/27252453/
- Alan D. Grinnell, Early milestones in the understanding of echolocation in bats. Journal of Comparative Physiology A 204 (2018), 519 to 536. https://pubmed.ncbi.nlm.nih.gov/29687162/
- Peter T. Madsen and Annemarie Surlykke, Functional convergence in bat and toothed whale biosonars. Physiology 28 (2013), 276 to 283. https://pubmed.ncbi.nlm.nih.gov/23997187/
- Bertel Møhl and others, The monopulsed nature of sperm whale clicks. J. Acoust. Soc. Am. 114 (2003), 1143 to 1154. https://pubmed.ncbi.nlm.nih.gov/12942991/
- Signe Brinkløv, M. Brock Fenton and John M. Ratcliffe, Echolocation in oilbirds and swiftlets. Frontiers in Physiology 4 (2013), 123. https://pmc.ncbi.nlm.nih.gov/articles/PMC3664765/
- Björn M. Siemers and others, Why do shrews twitter? Communication or simple echo-based orientation. Biology Letters 5 (2009), 593 to 596. https://pmc.ncbi.nlm.nih.gov/articles/PMC2781971/
- Lore Thaler, Stephen R. Arnott and Melvyn A. Goodale, Neural correlates of natural human echolocation in early and late blind echolocation experts. PLoS ONE 6 (2011), e20162. https://pmc.ncbi.nlm.nih.gov/articles/PMC3102086/
- Liam J. Norman, Caitlin Dodsworth, Denise Foresteire and Lore Thaler, Human click-based echolocation: effects of blindness and age, and real-life implications in a 10-week training program. PLoS ONE 16 (2021), e0252330. https://pmc.ncbi.nlm.nih.gov/articles/PMC8171922/
- Yossi Yovel, Michal Geva-Sagiv and Nachum Ulanovsky, Click-based echolocation in bats: not so primitive after all. J. Comp. Physiol. A 197 (2011), 515 to 530. https://pubmed.ncbi.nlm.nih.gov/21465138/
- Animal Diversity Web (University of Michigan), Eptesicus fuscus: FM calls of 1 to 5 ms from 50 to 25 kHz. https://animaldiversity.org/accounts/Eptesicus_fuscus/
- Animal Diversity Web, Euderma maculatum: calls of 9 to 12 kHz. https://animaldiversity.org/accounts/Euderma_maculatum/
- Bat Conservation Trust, Greater horseshoe bat: almost constant frequency call of about 82 kHz. https://www.bats.org.uk/about-bats/what-are-bats/uk-bats/greater-horseshoe
- Bat Conservation Trust, Brown long-eared bat (the whispering bat). https://www.bats.org.uk/about-bats/what-are-bats/uk-bats/brown-long-eared-bat
- Hans-Ulrich Schnitzler and Annette Denzinger, Auditory fovea and Doppler shift compensation: adaptations for flutter detection in echolocating bats using CF-FM signals. J. Comp. Physiol. A 197 (2011), 541 to 559. https://www.ebi.ac.uk/europepmc/webservices/rest/search?query=EXT_ID:20857119&format=json&resultType=core
- Arjan Boonman, Sara Bumrungsri and Yossi Yovel, Nonecholocating fruit bats produce biosonar clicks with their wings. Current Biology 24 (2014), 2962 to 2967. https://pubmed.ncbi.nlm.nih.gov/25484290/
- NASA Glenn Research Center, Speed of Sound. https://www.grc.nasa.gov/www/k-12/airplane/sound.html
- NOAA Ocean Service, What is sonar? https://oceanservice.noaa.gov/facts/sonar.html
- National Institute of Biomedical Imaging and Bioengineering, Ultrasound. https://www.nibib.nih.gov/science-education/science-topics/ultrasound
- Bosch Mobility, Ultrasonic sensor: detection range 15 cm to 5 m. https://www.bosch-mobility.com/en/solutions/sensors/ultrasonic-sensor/
- Absorption of sound in air: ISO 9613-1:1993, Acoustics, attenuation of sound during propagation outdoors, part 1 (formula used in the model).
- The sources for each animal and machine in the list under the stage are linked from its card.
More exhibits
How a music box works
A steel tooth 30.6 mm long rings at 261.6 Hz, and cutting it to half that length would raise the note two octaves.
How a phonograph works: from tinfoil to cassette and CD
Edison's first phonograph cut a voice into tinfoil in 1877, and the same needle played it back from a groove 2.54 mm apart.
How a piano works: the grand action and equal temperament
Press a key 10 millimetres and a felt hammer flies to the string, hits it and falls away before it can stop the note.
What sound looks like: sound waves, frequency and decibels
A 440 Hz tone packs the air into dense layers 78 centimetres apart, yet even at 94 dB each bit of air moves less than a thousandth of a millimetre.
How does a vinyl record work? Grooves, stereo and RIAA
At the outer edge of an LP the groove slides under the stylus at half a metre per second, and by the last song it has slowed to 21 centimetres.
How lightning and thunder work
A lightning channel heats the air to about five times the temperature of the Sun’s surface, and its thunder needs about 3 seconds to cover each kilometre to you.